
A family resemblance with important differences
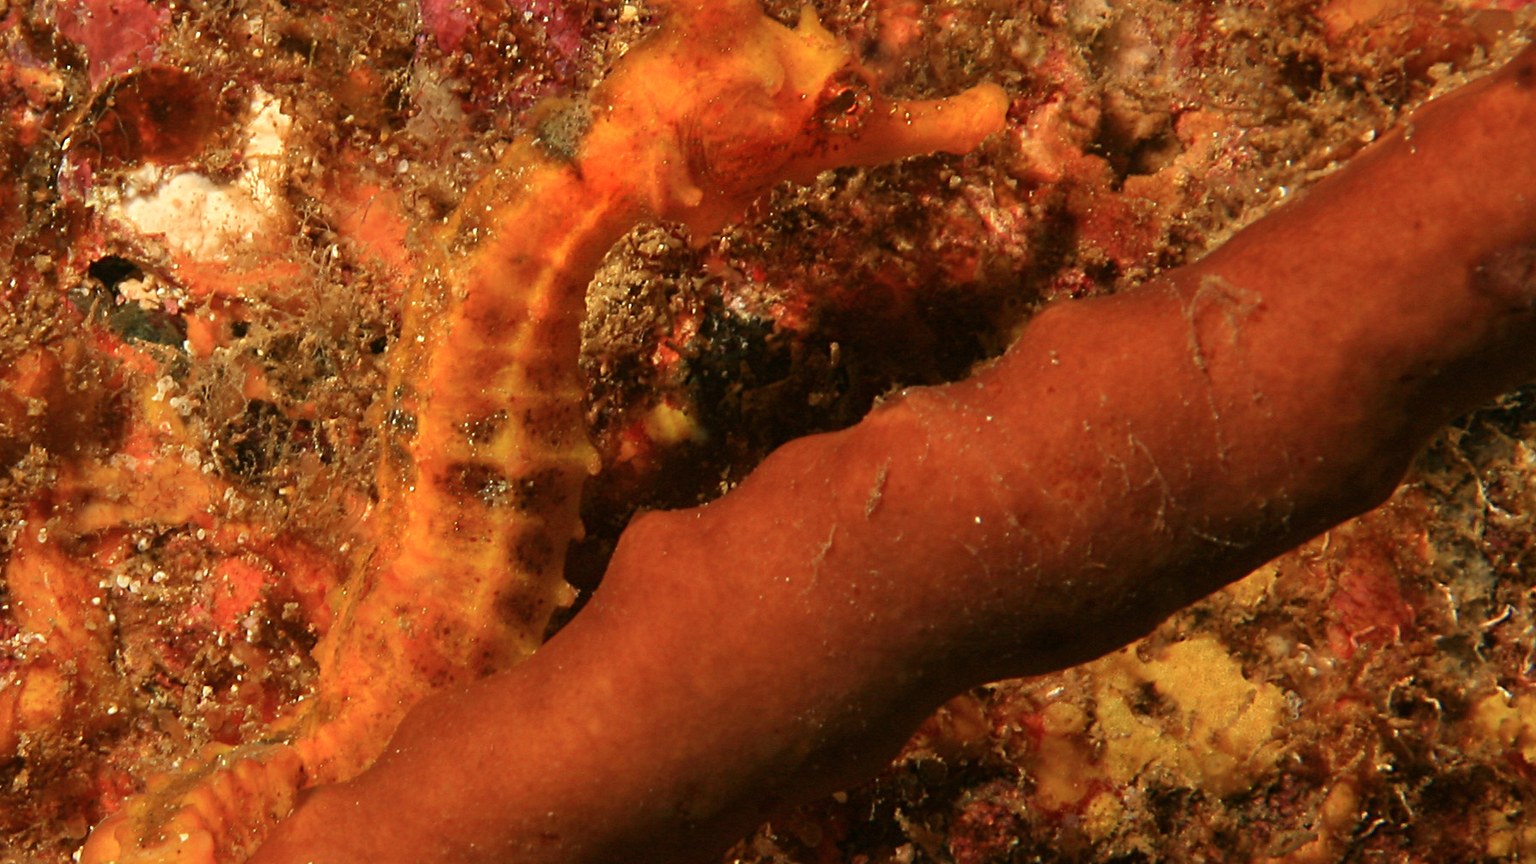
Seahorses are ray-finned bony fishes, despite their upright stance and horse-like profile. The name covers the genus Hippocampus, part of the family Syngnathidae alongside pipefishes, pipehorses and seadragons, within the order Syngnathiformes. An angled head and tubular snout sit above a body that can remain anchored by its gripping tail while the fish watches for prey. Identifying the genus is often easier than identifying the species. Closely similar forms and camouflage can obscure the features that separate one species from another. Names such as pygmy, spiny and common seahorse are applied to different named species, making the scientific name especially useful.
Snout proportions and body ornamentation help separate neighboring species. The long-snouted seahorse of the eastern Atlantic and Mediterranean, Hippocampus guttulatus, has a snout exceeding one third of its head length, angular bony tubercles and pale bluish-white spots or flecks. Fleshy strands can form a mane along its neck. The short-snouted H. hippocampus has a shorter muzzle and lacks those elongated neck protuberances. These structural differences offer more useful identification clues than a passing resemblance to the color of nearby vegetation.
Species boundaries also emerge from genetic comparisons. A revision combining morphology with mitochondrial COI evidence, published on 5 August 2026, recognized H. amandavincentae from Indian Ocean material, including southeastern India and genetic records from Madagascar, Mozambique and Seychelles. It has a relatively short snout, five coronet spines and spines along all principal trunk and tail ridges. In that revision, H. histrix in the strict sense is Pacific, including Japan, Indonesia and the Philippines. Northwestern Indian Ocean H. jayakari, originally described from the Gulf of Oman, has four cleithral spines, the lowest forked, and spines on alternating tail rings. Possible northern Red Sea overlap between H. amandavincentae and H. jayakari still needs targeted field confirmation.
The genus name is Hippocampus Rafinesque, 1810. WoRMS treats H. bleekeri as a synonym of H. abdominalis, so those two names do not identify separate species in that classification.
Armor that bends, fins that maneuver
Bony plates embedded beneath the skin form articulated armor. In the tail, successive rings of four L-shaped plates surround the vertebral axis. Their joints allow bending and twisting while preserving a protective framework around the backbone. The resulting tail is roughly square in cross-section and can curl around a holdfast. This combines two demands that might seem difficult to reconcile: an armored covering and the flexibility needed to grasp an irregular branch or blade.
A 2015 biomechanics investigation used seahorse anatomy, including scans of H. reidi, to build printed square and hypothetical cylindrical tail prototypes. The square design combined grasping with resistance to crushing through its plates and joints. In compression tests, six-segment square models were approximately three times as stiff and four times as strong as cylindrical models. Those ratios describe the printed structures under particular loads; the experiment did not measure the strength of living fish or their survival during predator attacks.
A dwarf seahorse, H. zosterae, maneuvers through coordinated movements of its dorsal and pectoral fins, while its swim bladder contributes to vertical stability. Its tail can hold seagrass or floating vegetation during a pause in swimming. Independently moving eyes help it search for prey from that position.
Sea fans, seagrass and deeper reefs
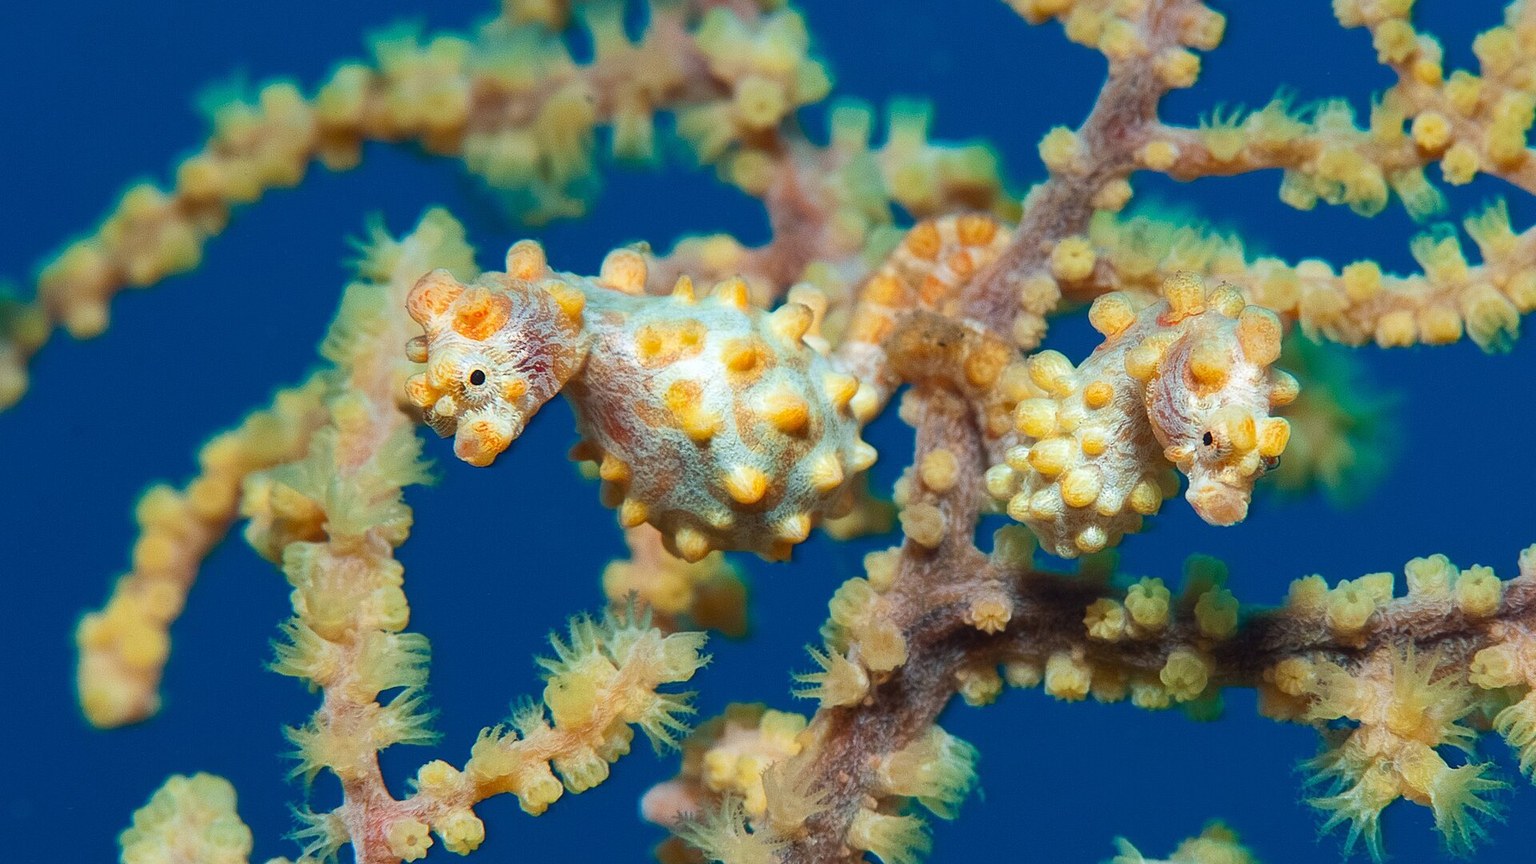
Bargibant’s pygmy seahorse, H. bargibanti, has a different silhouette: an extremely short snout, rounded coronet and bulbous tubercles that obscure the familiar ringed outline. It reaches about 24 millimetres in height. Its camouflage matches both the color and texture of its sea-fan host. Gray or purple fish with pink or red tubercles resemble Muricella plectana; yellow fish with orange or yellow tubercles resemble M. paraplectana. Its tail curls around the gorgonian branches on which it lives. The species was discovered on gorgonian material collected in New Caledonia in 1969; its resemblance to its host made even a collected sea fan capable of concealing this tiny vertebrate.
This pygmy inhabits tropical western Pacific reefs and slopes, including Indonesia, the Philippines, Japan, Papua New Guinea and the Great Barrier Reef, with records at 16–60 metres, usually on Muricella. Other seahorses occupy temperate vegetation: H. guttulatus occurs around southern England, southwestern Wales and Mediterranean coasts among algae and seagrasses. The great seahorse, H. kelloggi, has a compiled depth range of 1–150 metres and deep-water coral associations. Its Indo-West Pacific distribution extends from East Africa and the Red Sea region to Japan, New Caledonia and Australia. That span combines occurrences in different settings, rather than describing the preferred depth of every population.
On Australia’s east coast, White’s seahorse, H. whitei, ranges from Hervey Bay to Sussex Inlet, with important populations in Port Stephens and Sydney Harbour. It can reach 16 centimetres in length and has a long snout and tall, five-pointed coronet; individuals can change color between dark brown and pale tan. Named for John White, this estuarine species occupies depths of 1–18 metres. In Port Stephens, adults favor sponges, soft corals and Posidonia australis seagrass, while juveniles favor gorgonian fans as well as sponges and soft corals.
Sydney-region White’s seahorses also grip protective swimming nets, where encrusting growth supplies attachment habitat. Brazilian H. reidi similarly uses diverse structures. In the Linguado Channel of Babitonga Bay, Santa Catarina, fortnightly surveys from December 2021 to May 2022 found fish holding mangrove and fallen branches on one bank and metal fences and ropes on a developed bank. Fixed 20-by-2-metre transects were surveyed in water no deeper than one metre during ebb and low tides. Most behavioral records involved attached fish. These shallow, low-tide observations establish use of both settings; without measuring the availability of each structure, they do not establish a preference. Broader Brazilian surveys recorded anchoring on mangroves, macroalgae, cnidarians, seagrasses, sponges and bryozoans, with resightings consistent with restricted local space use.
Close-range hunters in a crustacean food web
The dwarf seahorse occurs along the US Gulf states, Mexico and parts of the greater Caribbean, including Cuba and the Bahamas, closely associated with seagrass and sometimes drifting vegetation. In a Thalassia testudinum bed near Tampa Bay, harpacticoid copepods dominated its diet by both item number and estimated biomass. The fish were sampled during daylight from April to October 1984 in water roughly 0.25–1 metre deep. The sampled water was 24–32 degrees Celsius. Comparing gut contents with crustaceans on seagrass blades connected prey consumption to the local feeding environment.
These tiny prey were assessed in two distinct ways. Researchers identified, counted and measured food throughout the dwarf seahorse’s tubular gut, which lacks a differentiated stomach. They estimated dry-weight biomass from prey size and weight relationships. Numerous small items and a few larger ones can contribute differently to those measures; in this case, harpacticoids predominated in both. Juvenile gulf pipefish, Syngnathus scovelli, shared the copepod resource but shifted toward larger amphipods and shrimp as they grew. Dwarf seahorses remained strongly dependent on harpacticoids across the sampled size classes.
Larger prey feature in the diet of wild adult H. abdominalis among Wellington Harbour macroalgae. Crustaceans dominated a 2002 gut-content study, including caprellid and ischyrocerid amphipods, the shrimp Hippolyte bifidirostris and the mysid Tenagomysis similis. Male and female diets did not differ in that population. Amphipod consumption peaked in spring and summer, while decapod consumption was lowest in autumn, showing seasonal changes within the same local food web.
Capturing a copepod demands more than waiting nearby. In laboratory trials with H. zosterae and Acartia tonsa, a relatively undisturbed region above the snout allowed close approach before a rapid head rotation and suction captured the prey. Observed strikes began only 0.5–1.4 millimetres away; the pivot covered that distance in less than one millisecond. The live-flow comparison involved 15 approaches by six fish. Water speeds in the strike region stayed at or below 0.8 millimetres per second, compared with 4.1 ± 1.5 in adjacent regions.
Preserved-specimen flow comparisons helped isolate the role of shape and posture. Seahorse heads produced reduced deformation near the strike region, whereas three-spined stickleback heads generated a relatively uniform bow wave ahead of the mouth. The quiet approach and sudden pivot explain how a slowly swimming predator can capture mobile prey at very short range. Seahorses themselves are food for larger animals: records include tuna and dorado stomach contents, as well as consumption by skates and rays.
The living work of a male brood pouch
The female produces eggs and transfers them to the male’s brooding structure; the male supplies sperm and carries the embryos until birth. Brooding anatomy varies within the genus. Larger familiar seahorses have a conspicuous pouch near the tail base, whereas the pygmy group exemplified by H. bargibanti broods within the trunk and has a single gill opening behind the head. Its small body therefore differs from estuarine H. whitei in reproductive anatomy as well as size and habitat.
Inside a pregnant H. abdominalis, the pouch’s exchange lining becomes more folded, capillary density increases and the distance from blood vessels to the pouch interior decreases. Greater surface area and closer vessels provide an architecture suited to respiratory gas exchange with developing young. A separate comparison of newly fertilized eggs and newborns found similar dry mass despite development’s energetic costs, supporting paternal nutrient supplementation alongside the yolk supplied by the female. These findings reveal an active developmental environment, with the scale of each contribution still incompletely quantified.
Birth also involves specialized anatomy. A 2022 investigation found large skeletal muscle bundles attached to modified anal-fin bones around the male H. abdominalis pouch opening. The proposed mechanism is that these muscles and body movements help open the pouch and expel newborns. Pouch tissue contained only scattered small smooth-muscle bundles, and isolated tissue did not measurably contract when exposed to isotocin in the experiment. Direct biomechanical testing is still needed to establish the proposed skeletal muscles’ role during birth.
Courtship, partners and reproductive timing
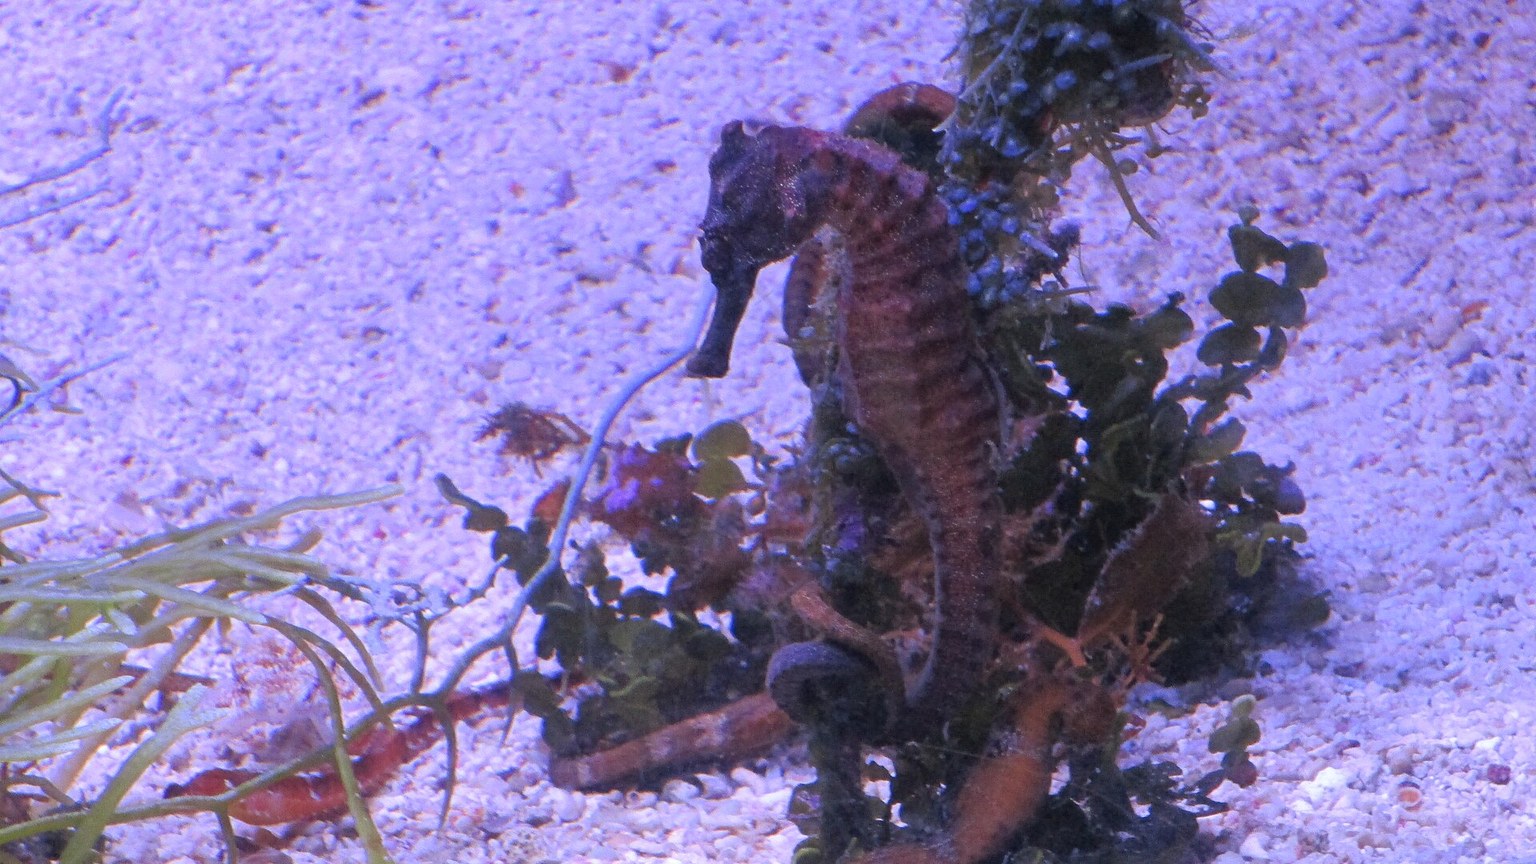
Wild Australian H. whitei pairs in an underwater study greeted daily and mated repeatedly and exclusively. Their bonds persisted across reproductive cycles and ended when a partner disappeared. H. abdominalis presents a different social pattern: a 2007 study recorded courtship with multiple partners, yet all genetically assayed broods had one mother and one father. Courtship participation and brood parentage describe different relationships. Female mating competition occurred in high-density, female-biased wild populations, while laboratory populations showed conventional sex roles. Partner fidelity therefore needs its species and population context; lifelong pairing is not a universal seahorse rule.
Sound accompanies some interactions. Male and female H. reidi produced clicks during feeding and courtship in a 2014 study, with most acoustic energy between 50 and 800 hertz. Clicks were most abundant on the third, final courtship day and particularly associated with male pouch pumping, a pattern consistent with reproductive coordination. During handling, fish also produced lower-frequency growls, concentrated below 200 hertz, together with body vibrations. Those observations establish when sounds occurred, while their communicative functions remain interpretations.
Reproductive schedules differ among species and settings. Wild H. whitei breeds from October to March in the NSW account, carrying pregnancies of about three weeks and releasing 100–250 young at a birth, with reproduction repeated up to eight times in a season. For H. zosterae, NOAA’s 2020 synthesis places maturity at about three months and reports experimentally observed gestation of 10–12 days; Tampa Bay field records include pregnant males in every month. Brazilian H. reidi surveys likewise recorded reproduction throughout the year.
Managed breeding reveals additional distinctions. In Tuticorin, India, adult H. kuda obtained as Gulf of Mannar bycatch produced six broods during August to November 2003, containing 162–317 young, averaging 262 ± 59. Newborns averaged 7.83 ± 0.35 millimetres in length and were reared at 26.5–28 degrees Celsius. Their sons showed courtship at 85–90 days after birth; males received eggs at approximately 101 ± 2 millimetres body length, while females transferred eggs at approximately 110 ± 2 millimetres. That offspring generation produced young 21–24 days after mating, with initial broods of 30–65 normal newborns. These first broods were smaller than those produced by the originally collected adults. Courtship, egg receipt and birth are separate milestones, and these managed observations do not establish wild ages at first reproduction.
Independent young and different lifespans
Released young feed independently, without continuing parental provisioning. Some species enter the water column after birth, offering a route for passive dispersal beyond the small breeding-season home ranges documented for many adults. H. bargibanti has a pelagic early phase; after it, the young settle on gorgonians and develop their enlarged tubercles and characteristic adult coloring. The duration and population-level importance of juvenile dispersal remain poorly resolved for many seahorses. Even after settlement, habitat use can change with age, as the differing holdfast associations of young and adult White’s seahorses illustrate.
Longevity is similarly species-specific. Wild H. zosterae rarely lives beyond two years in NOAA’s synthesis, although aquarium records reach three years. NSW reports wild H. whitei living up to six years. Field age estimates remain sparse across the genus.
Male care extends beyond seahorses within their family. The common or weedy seadragon, Phyllopteryx taeniolatus, carries eggs externally beneath the male’s tail. Its elongated body bears leaf-like appendages, unlike the upright seahorse outline and enclosed brooding arrangement. Native to temperate Australian waters from central New South Wales around the south coast to southwestern Western Australia, it lives on kelp-covered rocky reefs and eats small crustaceans such as mysids.
Conservation begins with attachment habitat
White’s seahorse is listed as Endangered under Australia’s EPBC Act. All syngnathids occurring in Australian waters also fall within the Act’s listed-marine-species category, a separate designation from threatened status. For H. whitei, storm scouring, freshwater floods, moorings and inappropriate swimming-net cleaning damage seagrasses, sponges, soft corals and encrusted attachment structures. Port Stephens suffered major habitat and seahorse losses after floods in 2021 and 2022, followed by further impacts in 2025.
Recovery work combines breeding and habitat provision. Sixty steel seahorse hotels installed in Port Stephens in 2023 supplied frames that marine organisms colonized above bare sand. Each measured one metre by one metre and 70 centimetres high, providing an elevated framework on which attachment habitat could develop. Seahorses continued to occupy algae- and sponge-covered hotels after the 2025 floods, while estuary-wide abundance remained very low. A completed 2022–2023 project released more than 300 captive-bred White’s seahorse juveniles into Port Stephens and Botany Bay, alongside cauliflower soft-coral restoration. Occupancy, releases and population recovery are distinct outcomes. Elsewhere, NOAA’s 28 July 2020 finding concluded that US Endangered Species Act listing of H. zosterae was not warranted at that time, following its February review.
Fisheries and international trade controls
Seahorse conservation also reaches working fisheries. A 2025 Philippine study based on 268 fisher and trader interviews conducted in 2019 across 17 coastal provinces documented catches through multiple methods and ongoing trade. It identified modified push-nets, called micro-trawls, and attributed a substantial share of estimated catch to compressor divers. These interview-derived estimates describe those fisheries in 2019, rather than present global landings.
All Hippocampus species entered CITES Appendix II on 15 May 2004, following adoption in 2002. Appendix II regulates international trade: exports ordinarily require permits supported by scientific non-detriment findings concerning the effects of export on the species’ survival, and imports require presentation of the export permit or re-export certificate. Qualifying trade can occur under the applicable conditions. EU Regulation 2026/1383, dated 22 June and published on 26 June 2026, places the genus in Annex B. EU import assessment considers conservation effects on the species and the range occupied by the relevant population, trade levels and scientific review opinions.
Treaty obligations also have exceptions. The CITES reservation table effective from 5 March 2026 records genus-wide reservations by Indonesia, Japan and Norway, and reservations for H. denise and H. kuda by Palau. National laws, suspensions and transaction-specific exemptions add further conditions. These controls operate alongside habitat protection and fisheries management; they do not constitute a universal ban on every seahorse transaction.